www.sciencemag.org/cgi/content/full/316/5821/120/DC1
akiba-online 时间:2021-03-20 阅读:()
SupportingOnlineMaterialforAnATPGateControlsTubulinBindingbytheTetheredHeadofKinesin-1MariaC.
Alonso,DouglasR.
Drummond,SusanKain,JuliaHoeng,LindaAmos,RobertA.
Cross1**Towhomcorrespondenceshouldbeaddressed.
E-mail:r.
cross@mcri.
ac.
ukPublished6April2007,Science316,120(2007)DOI:10.
1126/science.
1136985ThisPDFfileincludes:MaterialsandMethodsSOMTextFigs.
S1toS4ReferencesPageS1SSupplementaryMaterial|Alonsoetal|ATP-GatingmechanismofKinesinSupplementaryMethods1.
Proteins&proteinchemicalmethods1.
1Proteins|Nkin460GSTcontainingtheN-terminal460aminoacidsofNeurosporakinesin-1andaC-terminalGSTfusionwaspreparedasdescribed(1).
Rat430GSTprotein(2)usedinthesteadystateATPaseassayscontainedtheequivalent430N-terminalaminoacidsofratKinesin-1andaC-terminalGSTfusion.
ThisproteinwasagiftfromDrIsabelleCrevel.
RatrK430asusedintheFPLCgelfiltrationandthekineticsexperimentswasuntagged.
TheinsertforthisconstructwasPCRamplifiedfromafulllengthratkinesin(kif5cclone)originallygiventousbyScottBrady.
StartingOligo:5'-CCGCTCTACATATGGCGGACCCAGCCGAATGCAGC-3'EndingOligo:5'-CCGACTAGTCTAGAATTCCTTGTCATCCAGCTG-3'.
ThePCRproductwasdigestedwithNdeI/SpeIandligatedintopET17b.
Expressionandpurificationoftheproteinwasaccordingto(3).
PigbraintubulinwaspreparedaccordingtoMitchisonandKirschner(4)(http://mitchison.
med.
harvard.
edu/protocols.
htm)andS.
pombetubulinbyamodificationofthemethodofDavisetal(5)tobedescribedindetailelsewhere.
PurifiedtubulinsweredesaltedintoPEMcontaining20μMGDPbeforestorageinliquidnitrogen.
ProteinconcentrationsweredeterminedbyUVabsorptionscanofsamplesofproteindissolvedin6Mguanidinehydrochloride,correctingforbackgroundscatteringbysubtractingascanofbufferalone,andassumingfullnucleotideoccupancy.
1.
2SteadystateATPase|ThemicrotubuleortubulinheterodimerstimulatedATPaseactivityofkinesinwasmeasuredat25Cusingapyruvatekinase/lactatedehydrogenaselinkedassayasdescribed(6),exceptthatmicrotubuleswereassembledinPEM(7)containing1mMGMPCPP,pelletedandresuspendedinPEMcontaining10nMGMPCPPbeforedilutionintothelinkedassaybuffer(20mMPIPES,pH6.
9,5mMMgCl2,1mMDTT,0.
1mgml-1BSA).
TubulinheterodimersweredilutedfromastockinPEMcontaining20μMGDP.
NAD/HabsorptionmeasurementsweremadeinaCary50spectrophotometerusingdisposable50μlUVtransparentcuvettes(Eppendorf).
ValuesforVmaxandKmwereobtainedbyleastsquaresfittingtoplotsofATPaseversustubulinheterodimerconcentration,usingKaleidagraph3.
6.
4(SynergySoftware).
ATPasevaluesareperkinesinhead.
1.
3Superose12gelfiltration|Stockkinesin(typically69Mheadsconcentrationin20%glycerol,20mMphosphatebufferpH7.
0,2mMMgCl2,0.
3MNaCl,0.
1mMDTT)wasmixedwithstocktubulin(typically58μMheterodimersin50mMPIPESpH6.
9,0.
2mMMgCl2,1mMEGTA,0.
1μMNa-GTP,30%glycerol)andadjustedtoafinalvolumeof240landfinalconcentrationsof6.
5μMkinesinheadsand13μMtubulinheterodimers,witheithernoaddednucleotide,or2mMAMPPNPor2mMADPbyadding10xcolumnbufferandwaterasnecessary.
Themixturewasincubatedfor10minsoniceandcentrifugedbrieflyinamicrofuge(thiswasprecautionary:nopelletwasobtained).
Theentire240μlsamplewasthenappliedtoaSuperoseHR10/300GLcolumnheldat4Candrunningat0.
5mlmin-1.
Thecolumnbufferwas50mMPIPESpH6.
9,2mMMgCl2,1mMEGTA;pluseithernothingor2mMADPor0.
2mMAMPPNP.
0.
3mlfractionswerecollected.
ThereducedconcentrationofAMPPNPinthecolumnbufferwasfoundtobeadequateandwasusedforreasonsofcost.
Elutionpatternsweremonitoredat290nmtoavoidthelargenucleotidecontributiontothe280nmabsorbance.
ThekinesinabsorbanceislowbecausetherearefewtryptophansintherK430sequence.
Thisisconvenientbecauseitmeansthatthetubulinbehaviourdominatestheelutionprofilesfromthemixtures.
PageS2S1.
4Gelelectrophoresisanddensitometry|SamplesfromthepeakfractionswererunonInvitrogenNuPAGE10%bis-trisprecast15wellgelsandruninMOPS(Invitrogen)bufferat200Vfor1.
5hours.
GelswerestainedwithSimplyBlue(Invitrogen)andimagedwithagreyscaleCCDcamera.
QuantitationwasinitiallydoneusingImageJ(Rasband,W.
S.
(1997-2006);http://rsb.
info.
nih.
gov/ij).
Integratedopticaldensityvaluesforeachbandwerecorrectedbysubtractingtheintegratedopticaldensityofacorrespondinglocalareaoffeaturelessgel.
Thesystemwascalibratedusinganopticaldensitywedge.
Inlaterwork,weusedthesyproorgangefluorescentstainingsystem(MolecularProbes,methodexactlyaspermanufacturer'sinstructions)incombinationwithaPhosphorimager(MolecuarDynamics)andBioRadImageQuantsoftware.
Thetwoapproachesgavecomparableresults.
ThenumbersquotedinthetextreferonlytothePhosphorimager/Syproreddata.
1.
5MantATPturnoverexperiments|Stocktubulin(seeabove)wasdialysedfor30minutesagainstalargeexcessvolumeof50mMPIPESpH6.
9,0.
2mMMgCl2,1mMEGTA,10%glyceroltoremoveunboundguanidinenucleotides.
TheconcentrationofthedialysedproteinwasdeterminedbyUVabsorptionscan(seeabove).
Enzymereactionsweredonein20mMPIPESpH6.
9,2mMMgCl2,usingquartzfluorimetercuvettes.
FluorescencetransientswererecordedwithaCaryEclipsefluorimeter.
Atthestartofthereaction,cuvettescontained1μMMantATPin20mMPIPESpH6.
9,2mMMgCl2.
Tothisweaddedkinesintoafinalconcentrationof1μMkinesinheads,andinsomeexperimentstubulintoafinalconcentrationof2μMtubulinheterodimers.
Thenwe"chased"byaddingeither100mMNa-ATPor100mMAMPPNP,to1mMfinalconcentration.
Thefinalvolumeineverycasewas600μl.
Experimentsinwhich4Moftubulinwasaddedyieldedessentiallyidenticalresults(notshown).
PageS3S2.
SupplementaryData.
2.
1Superose12gelfiltrationofkinesin-tubulinmixturesFigureS1|Superose12chromatographyofkinesin-tubulinmixturesThedatawereobtainedasdescribedaboveandforFig.
2inthemaintext,andtheaxesareequivalent.
Thedifferenceinthiscaseisthatamixingratioof1tubulinheterodimerperkinesinheadwasused.
Thetubulinpeak(therightmostpeakvisibleinFig.
S1AandFig.
S1B)isthenentirelyshiftedtoanearlierelutionpositioninFig.
S1C.
PageS4S2.
2Dockingtubulinheterodimerstotheratkinesindimer(3KIN)crystalstructureFigureS2(below)showsthatthetubulinbindingsitesof3KINarepositionedsothatweretubulinheterodimerstobindtothisstructure,theywouldbespacedwellapartandwouldnotclashwithoneanother.
In3KIN,bothheadsareoccupiedbyADP,andbothnecklinkersaredocked.
OurdatashowthatonlyonetubulinheterodimercanbindtoakinesindimerintheabsenceofAMPPNP.
FittingofcryoEMdatasuggeststhepossibilitythatthetubulinbindingsiteinthesecondheadisphysicallymasked(below).
Furtherworkwillberequiredtodeterminethestructuralmechanismbywhichthetubulinbindingsiteonthesecondheadisblocked.
FigureS2|Dockingtubulinheterodimerstotheratkinesindimer(3KIN)crystalstructurePageS5S2.
3Dockingakinesincrystalstructureintotheparkedheadofacryo-EMstructureThemicrotubuleboundheadThecryo-EMsurfacecontourmapshowninFig.
S3isof15-pfMTsdecoratedwithdimericratkinesin-1intheabsenceoffreenucleotide(8),expectedtocorrespondtotheATP-waitingdwellstateinthewalkingmechanism.
Thismaphasaresolutionof~30.
SupplementaryFigs.
S4A-Cshowdockingofamodelcomprisingatubulinprotofilamentwithonekinesinheadbound(whitepolypeptidebackbone)intotheCryoEMmap(bluenet).
ThismodelcomplexcomprisestubulinandthemotordomainofKar3inanorientationderivedinseparateexperimentsbydockingintoahighresolutioncryo-EMmap(9).
Themaincontactwithtubulinismadebyhelixα4ofthemotordomain,aswasalsofoundforKif1A(10).
Thecrystalstructuresofkinesin-1'scanbealignedtothoseofKar3withr.
m.
s.
differencesof1.
5-3,sothetubulin-Kar3complexservesasasufficientmodelhere.
ThetetheredheadWethenconsideredthepositionofthesecond(tethered)head.
Fittingwasdonebyeyeusingoneheadoftheratkinesindimer3KIN,requiringthatthetwostrandsofthecoiledcoilneckofthedimerremainclose.
Figs.
S4A-Cshowthetetheredheadingreen.
Thisapproachyielded2possibledockingsforthesecondhead,AandB.
Boththesedockingsforthesecondmotordomainhavetheα-helicalneckofthesecondmotordomaininroughlytherightregiontopairintoacoiledcoilwiththatofthefirstmotordomain.
Fig.
S4Ashowsthefrontviewofthesetwoalternativefits.
ItisclearthatdockingAprovidesthebetterfit.
Yellowarrowspointtothestretchofhelixthatwouldformhalfofthecoiled-coilstalk.
Thedifferencesbetweenthedockingsarelessdistinctinotherviews(Fig.
S4B&S4C)sincetheoverallshapeofthemotordomainisroughlytriangular,withupto6possibledockings.
CaveatIndoingthisfitting,weconsideredthepossibilitythatthebulkofthekinesin-1motordomainmaymoverelativetoα4,ashasbeenobservedforKif1A(10,11),butnotforKar3(9).
Ifsuchamovementoccurred,itwouldnoticeablyaffectthepositionofthealphahelicalcoiledcoilstalkbutnotthespaceavailablefordockingthe2ndhead.
TheworkonKar3suggeststhatthetopoftheboundmotordomainundergoesasignificantconformationalchangeintheapostatebutthereisnocrystalstructureforthisstate.
Accordingly,thepossibilitythatthemainpartoftheheadmightshiftrelativetoalpha4limitstheprecisionofthefitting.
Specifically,thereisuncertaintyabouttheprecisepositionoftheendofthenecklinkerofthethemicrotubule-boundhead.
Nonethelesstheapproximatefitobtainedisrobust,becausetheelongatedshapeoftheheadincombinationwitharequirementforcloseappositionofthetwonecksprovidesasufficientconstraint.
PageS6SConclusionsHigherresolutionstudiesoftubulinanddimerickinesinarerequiredtoestablishthepreciseandunequivocalorientationforthesecondhead.
Itisnonethelessclearthatthemostreasonablefit(dockingA),leadstopartialocclusionofthemicrotubulebindingsurfaceofthetetheredhead,suggestingthattubulinbindingbythetetheredheadisinhibitedinthedwellstatebyparkingthetetheredheadagainsttheboundheadsoastomaskitstubulinbindingsite.
AlonsoetalSupplementaryFig.
S3.
CryoEMmapofthedwellstate(8)PageS7SAlonsoetalSupplementaryFig.
S4.
FittingthecryoEMmap.
Fig.
S4A|FrontViewDockingADockingBPageS8SFig.
S4B|SideViewDockingADockingBPageS9SFig.
S4C|TopViewDockingADockingBSupplementaryReferences1.
I.
Crevel,N.
Carter,M.
Schliwa,R.
Cross,EmboJ18,5863(1999).
2.
I.
M.
Crevel,A.
Lockhart,R.
A.
Cross,JMolBiol273,160(1997).
3.
A.
Lockhart,I.
M.
Crevel,R.
A.
Cross,JMolBiol249,763(1995).
4.
T.
Mitchison,M.
Kirschner,Nature312,232(Nov15-21,1984).
5.
A.
Davis,C.
R.
Sage,L.
Wilson,K.
W.
Farrell,Biochemistry32,8823(Aug31,1993).
6.
A.
Lockhart,R.
A.
Cross,EmboJ13,751(1994).
7.
J.
W.
Walker,G.
P.
Reid,J.
A.
McCray,D.
R.
Trentham,JAmChemSoc110,7170(1988).
8.
K.
Hirose,J.
Lowe,M.
Alonso,R.
A.
Cross,L.
A.
Amos,MolBiolCell10,2063(1999).
9.
K.
Hirose,E.
Akimaru,T.
Akiba,S.
A.
Endow,L.
A.
Amos,MolCell23,913(Sep15,2006).
10.
R.
Nitta,M.
Kikkawa,Y.
Okada,N.
Hirokawa,Science305,678(Jul30,2004).
11.
M.
Kikkawa,N.
Hirokawa,EmboJ(Aug31,2006).
tubulin
- www.sciencemag.org/cgi/content/full/316/5821/120/DC1相关文档
- assemblyakiba-online
- 周游akiba-online
- 补票akiba-online
- assessmentakiba-online
- ALTWakiba-online
- 2.2akiba-online
统计一下racknerd正在卖的超便宜VPS,值得推荐的便宜美国VPS
racknerd从成立到现在发展是相当迅速,用最低的价格霸占了大部分低端便宜vps市场,虽然VPS价格便宜,但是VPS的质量和服务一点儿都不拉跨,服务器稳定、性能给力,尤其是售后方面时间短技术解决能力强,估计这也是racknerd这个品牌能如此成功的原因吧! 官方网站:https://www.racknerd.com 多种加密数字货币、信用卡、PayPal、支付宝、银联、webmoney,可...
wordpress外贸企业主题 wordpress经典外贸企业建站主题
WordPress经典外贸企业建站主题,经典配色扁平化简约设计+跨屏自适应移动端设备,特色外贸企业建站功能模块+在线Inquiry询单功能,更有利于Google等英文搜索优化和站点收录。采用标准的HTML5+CSS3语言开发,兼容当下的各种主流浏览器: IE 6+(以及类似360、遨游等基于IE内核的)、Firefox、Google Chrome、Safari、Opera等;同时支持移动终端的常用...
快云科技,免云服务器75折优惠服务器快云21元/月
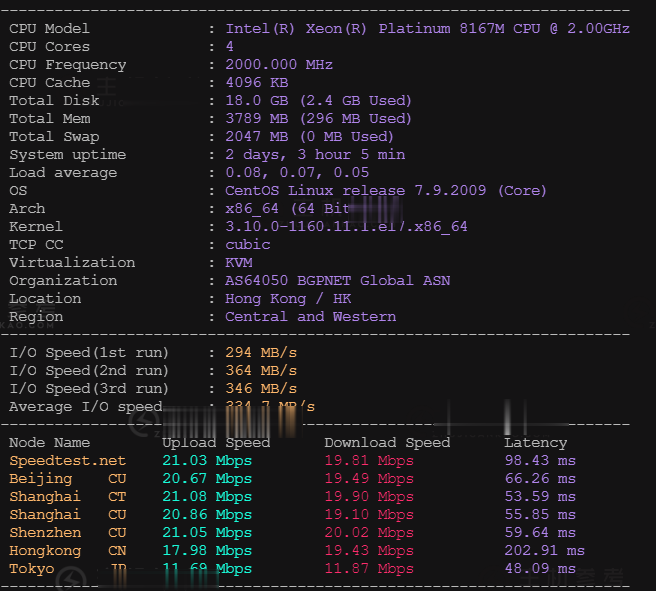
近日快云科技发布了最新的夏季优惠促销活动,主要针对旗下的香港CN2 GIA系列的VPS云服务器产品推送的最新的75折优惠码,国内回程三网CN2 GIA,平均延迟50ms以下,硬件配置方面采用E5 2696v2、E5 2696V4 铂金Platinum等,基于KVM虚拟架构,采用SSD硬盘存储,RAID10阵列保障数据安全,有需要香港免备案CN2服务器的朋友可以关注一下。快云科技怎么样?快云科技好不...
akiba-online为你推荐
-
编程小学生惊库克少儿编程,编程小将的班值得报吗?haole018.comhttp://www.haoledy.com/view/32092.html 轩辕剑天之痕11、12集在线观看www.kanav001.com长虹V001手机小游戏下载的网址是什么机器蜘蛛有谁知道猎人的机械蜘蛛在哪捉的苗惟妮和空姐一起的日子23集全集在线看下载电视剧分集剧情介绍红玉头冠wow里面达拉然那个鼎鼎有名的佛罗佐的头部是什么啊?就是三颗冰晶的那个,我记得是可以得到的、因为看剑影绝杀三国战记武将争霸中鬼剑士,曹操,吕布等人的大绝杀怎么发呀,速求百度关键词百度关键词24小时快排是怎么做的?为什么非要在前2页?大虫手绘古代人称的"大虫"是什么?www.533.cc一一影院最新网址是不是www.11dy.cc ?